Showing posts with label Cold Seeps. Show all posts

Sunday, 5 January 2025

Provanna dongshaensis: A new species of fossil Gastropod from hydrate-bearing sediments in the South China Sea.

The Abyssochrysoidea are a large group of Caenogastropods found in deep-sea environments. The genus Provanna is the largest within this group, currently containing 29 extant species from  hydrothermal vents, hydrocarbon seeps, and organic falls (such as sunken wood and Whale falls) in the Pacific Ocean, the Caribbean, the Southern Ocean, and off the west coast of Africa, as well as nine species from preserved seep deposits and organic falls in Japan, New Zealand, the United States, and Peru, the oldest of which date back to the Cretaceous. These Snails are grazers and detritivores form part of biological communities which are dependent on the chemosynthetic activities of Bacteria and Archaeans for their survival.

In a paper published in the journal Zoosystematics and Evolution on 2 January 2024, Cong Wu and Fang Chen of the National Engineering Research Center of Gas Hydrate Exploration and Development, the Key Laboratory of Marine Mineral Resources of the Ministry of Land and Resources, and the Guangzhou Marine Geological Survey, Ying Tian of the Key Laboratory of Mariculture and Stock Enhancement in North China Sea at Dalian Ocean University, and the Dalian Shell Museum, Kazutaka Amano of the Department of Geology and Paleontology at the Japanese National Museum of Nature and Science, and Xin Su of the School of Ocean Sciences from the China University of Geosciences, describe a new species of Provanna from specimens recovered from two drill cores sunk into cold seeps in the South China Sea.

The new species is described from two specimens, and three other shell fragments, recovered from two separate drill cores (GMGS2-09B and GMGS2-07B) sunk into the seafloor of the northern South China Sea. The shells were obtained from carbonate layers with carbon isotope signatures which strongly indicate that they were laid down at ancient methane seeps. The new species is named Provanna dongshaensis, where 'dongshaensis' means 'from Dongsha' in reference to the island known as 'Dongsha' in Chinese, which lends its name to the area where the fossils were found. This island is currently administered by Taiwan under the name 'Tungsha', and is known as 'Pratas Island' in English.

Global distribution of genus Provanna displayed as type locations of known species and location of the study (GMGS2-07B and GMGS2-09B). orange circle: active hydrothermal vents, hydrocarbon seeps where extant Provanna species are discovered; blue circle: seep deposits or organic falls that yield fossil Provanna. Wu et al. (2025).

The larger of the two specimens of Provanna dongshaensis is 10.89 mm high and has a final whorl width of 7.13 mm; the smaller has a height of 7.80 mm and a final whorl width of 5.02 mm. It is not possible to tell the length of the original shells as both are slightly damaged and lack their tips. This means that the protoconch (the shell that a marine Gastropod uses during its larval, planktonic stage), an important diagnostic tool for Gastropods is missing. Nor is the radula (tongue), another key diagnostic feature, present in any specimens, nor any genetic organic material from which DNA could be extracted. Previous studies, however, have established that the shell microstructure of the genus Provanna, is distinctive, so Wu et al. are confident in their assignment of the shells.

Provanna dongshaensis, from a late Pleistocene seep site in the northern South China Sea. (A)–(C) Holotype, GMGS2-09B-C15-2, specimen from core 09B-4, shell height: 7.8mm; (D)–(F) Paratype, GMGS2-07B-A1, specimen from core 07B-2H-2A with the protoconch almost lost, shell height: 10.89mm; (G)–(I) Incomplete specimen GMGS2-09B-C15-1 from core 09B-2M-1A; (J)–(L) Incomplete specimen GMGS2-09B-C14 from core 09B-4. (M)-(O) Incomplete specimen GMGS2-09B-C13 from core 09B-2M-1A. Scale bar is 5 mm. Wu et al. (2025).

The largest of the specimens in the collection has been dated to 91 693 yeats before the present, though all others are significantly younger, with dates of 16 230±50 years before the present and 15120±50 years before the present. This places all specimens within the final Pleistocene glaciation, although their chronological distribution is probably more closely linked to the life cycle of the cold methane seep where they lived than to the climate on the surface. Wu et al. note that a number of other Gastropod shells are present in the cores from which Provanna dongshaensis was derived, suggesting that the site might be significant for our understanding of ancient cold seeps in the South China Sea.

See also...

Wednesday, 20 October 2021

Investigating the drivers of methane release from cold seeps on the Southern Hydrate Ridge off the coast of Oregon.

Cold seeps release methane along most coastal margins, either as gas dissolved in water or as bubbles which rise through the water column. Bubbles of methane released from cold seeps have been observed rising hundreds of meters through the water column in the Guaymas Basin in the Gulf of California, on the continental rise off the coast of the Carolinas, along the Cascadia Margin off the coast of British Colombia and the northwestern US, in the Okinawa Trough in the East China Sea, in the Black Sea, and in the Gulf of Mexico, as well as at an experimental station in Monterey Bay. When emitted at depths of less than a hundred metres, methane bubbles typically reach the surface and release their gas into the atmosphere, while bubbles released at greater depths the methane in them is lost into the water column as they rise. However, in areas where stable gas hydrates exist at deeper depths, then the bubbles may have a hydrate coating, which slows dissolution of their gas content, allowing bubbles from greater depths to reach the surface. 

This gas is thought to be of minor significance compared to other sources of carbon entering the atmosphere, but the amount gas produced, and how this varies both geographically and over time, has been the subject of very little investigation. The amount of gas released at different sites is known to vary considerably, which is thought to be related to factors such as the subsurface structure and the source of the methane. External factors are also thought to affect the amount of methane being released, such as variations in hydrostatic pressure caused by the action of tides, swell, or storms, changes in sea temperature linked to seasons or longer term changes, seismic tremors, and even to isostatic rebound.

Hydrate Ridge forms part of the Cascadia Subduction Zone, an anticlinal ridge on the accretionary wedge with a north-south orientation. This ridge has two distinct areas of cold seeps, known as the Northern and Southern Hydrate Ridges, both of which have extremely large methane hydrate deposits close to the sediment surface, which lead to persistent gas emissions in the form of bubble plumes, as well as extensive chemosynthetic ecosystems and authigenic carbonates. Seismic profiling of the Southern Hydrate Ridge has found a reflective surface, thought to be the base of the gas hydrate zone, at 125 m beneath the sediment surface. This hydrate zone overlies a structure called Seismic Horizon A, along which methane-rich fluids appear to migrate from the underlying accretionary wedge. Bubble plumes are extremely visible here, and have not been shown to fluctuate with tidal cycles, as is the case on the Northern Hydrate Ridge. Instead, the rate of bubbling appears to follow a cycle unrelated to the tides. It has been suggested that this might be caused by the formation of gas hydrate seals close to the surface, which remain in place until the amount of gas accumulated in the sediment beneath them overcomes their resistance, then reform when gas emissions tail off sufficiently, a cycle which can take several years to complete. More recent surveys have established that while bubbling is not constant on the Southern Hydrate Ridge, it does appear to occur consitently at the same sites on the ridge, and can vary on an hourly timescale. This unexpected behaviour has led to a need for a more organised long-term monitoring of this system in order to understand it.

The systematic monitoring of activity has been carried out at several cold seeps, including a study on Clayoquot Slope, off the coast of Canada on the northern Cascadia Subduction Zone which lasted over a year, although the equipment used in that study was only able detect gas emissions when bottom currents were flowing in certain directions, hampering understanding of the system.

In a paper published in the journal Geochemistry, Geophysics, Geosystems on 21 September 2021, Yann Marcon of the Center for Marine Environmental Sciences and Department of Geosciences at the University of Bremen, Deborah Kelley of the School of Oceanography at the University of Washington, Blair Thornton of the Centre for In Situ and Remote Intelligent Sensing at the University of Southampton, and the Institute of Industrial Science at the University of Tokyo, and Gerhard Bohrmann, also of the Center for Marine Environmental Sciences and Department of Geosciences at the University of Bremen, present the results of a project that carried out systematic monitoring of the Southern Hydrate Ridge between July and November 2018.

Marcon et al. monitored gas emissions on the Southern Hydrate Ridge with the Southern Hydrate Ridge Rotating Sonar, which consists of a multibeam echosounder mounted on a rotator, with a rotating range of 360°. In addition they used a single-beam scanning-sonar connected to the Ocean Observatories Initiative's Regional Cabled Array to provide a finer detail monitoring gas releases at Einstein’s Grotto, one of the methane vents on the Southern Hydrate Ridge, and photo cameras also connected to the Regional Cabled Array to provide visual ground-truthing information about the dynamics and strength of bubble release, at Einstein’s Grotto and the Summit-A vent area. 

 
Top left: Location of Southern Hydrate Ridge. Top right: Map of the primary infrastructure of the Ocean Observatories Initiative's Regional Cabled Array observatory. Bottom: Overview map of the Southern Hydrate Ridge summit with the location of the Southern Hydrate Ridge Regional Cabled Array fibre optic cables, junction boxes and monitoring instruments. Shaded areas show the location of the main known vents. Marcon et al. (2021).

The bathymetry (depth of water) of the area was established in 2008 by the Autonomous Underwater Vehicle Sentry, operating from the Research Vessel Thomas G. Thompson, during preparation for the laying of the Ocean Observatories Initiative's Regional Cabled Array. A 3D photomosaic of the area was developed from imagery gathered by the University of Tokyo's Autonomous Underwater Vehicle AE2000f during the Schmidt Ocean Institute's FK180731 #Adaptive Robotics expedition.

A conductivity, temperature, and pressure (CTP) probe equipped with a dissolved oxygen optode sensor was used to monitor the conductivity, temperature, pressure, and dissolved oxygen concentration of the bottom water at one minute intervals. High-frequency tidal seafloor pressure was recorded with a tsunami pressure sensor. Current velocities were monitored with an upward-looking acoustic Doppler current profiler. Seismic data was collected by three ocean-bottom seismometers connected to the Regional Cabled Array. Wave height data was obtained from the National Data Buoy Center of the National Oceanographic and Atmospheric Administration.

Seafloor pressure at the Southern Hydrate Ridge was found to vary considerably with the tide, and was sensitive to the neep/spring tide cycle, with pressure varying by 1.4 dbar during neap tides and up to 3.8 dbar during spring tides. The seafloor temperature varied between 3.8°C and 4.5°C over the course of the study (June-November 2018) and between 3.7°C and 4.7°C over the longer period June 2018-June 2020, showing no long-term warming or cooling trend. Seafloor salinity varied between 34.26 to 34.37 psu over the period June-November 2018, while dissolved oxygen varied between 0.24 and 0.30 ml/L.

The Southern Hydrate Ridge Rotating Sonar carried out scans every two hours during the four month period of the experiment (with some gaps due to technical problems), producing a total of 888 readings. Of these, 886 (99.8%) detected gas bubbles, suggesting that bubbling was more-or-less constant. However, the amount of bubbling varied continuously, with peaks and troughs on a twice daily basis. These peaks and troughs appear to become larger at the spring tides and weaker at the neap tides, although the short duration of the experiment combined with the gaps in the data make it difficult to be completely confident about this.

Bubbling appears to be possible at any recorded pressure on the Southern Hydrate Ridge, although it was more pronounced when the pressure was low or falling. Two thirds of all peaks in activity occurred at times when the pressure was below average. The majority (65-70%) of the remaining third of peaks happened when the tide was decreasing, or changing (18-20%), with only a small proportion (15%) occurring while the tide was rising. However, there were some anomalies with this, most notably a large bubble release in July 2018m which occurred during a rising tide when the water pressure was above average.

 
Temporal variations of the Southern Hydrate Ridge Rotating Sonar backscatter magnitude and bottom pressure between 6 and 22 July 2018 (top plots) and between 19 October and 8 November 2018 (bottom plots). The backscatter magnitude non-linearly reflects the strength of the gas bubble emissions. The bottom pressure plot shows the local mixed tidal regime with diurnal and semi-diurnal constituents, as well as the fortnightly neap/spring tidal cycles. Bubble release is commonly stronger during ebb tide, and possibly also during spring tidal phases. However, some ebullition events do not correlate with the tide and may be triggered by local accumulation of pressurized free gas in the subsurface; the prominent peak observed on 18 July 2018 corresponded to the reactivation of the Summit-A vent after a very short venting interruption of about 4 hours; it did not affect the other vents at the Southern Hydrate Ridge summit and happened during flood tide within a neap tidal phase, hinting at shallow, local changes in the sediments. Marcon et al. (2021).

Eight different centres of bubbling were identified on the Southern Hydrate Ridge, with an average of four active at any given time. Five main clusters of activity were identified; each of these being 10-30 m across, and capable of producing more than one stream of bubbles at a time. These were named Smokey Tavern, Einstein's Grotto, Summit-A, Summit-B, and Summit-C. Bubbling at all of these sites was frequent, but not continuous, with sites remaining dormant for days at a time and all sites being active at the same time being a rare occurrence. As well as these main sites of activity around the summit of the Southern Hydrate Ridge, Marcon et al. detected at least six smaller venting sites, further away from the summit and much less active, which they named Smokey Tavern West, Summit-D, Far NE, Far S, Summit South, and Summit SW. Unlike the main sites, these sites were only sporadically active, and would often remain dormant for months between bouts of venting.

 
(a) Location of flare base points recorded with the Southern Hydrate Ridge Rotating Sonar between 8 July and 8 November 2018; the base points are grouped into clusters marking the location of the different Southern Hydrate Ridge vent sites. (b) Location of the main and periphery vents overlain on the photomosaic; the main vent sites are all located on areas covered with microbial mats. (c) Close-up view of the Southern Hydrate Ridge Rotating Sonar location and the Summit-A vent, with the 3D photomosaic in the background; a depression on the seafloor from Ocean Drilling Program drill site 1949 (ODP Leg 204) can be seen in the top-left corner as well as in the bathymetric data. (d) Close-up view of the 3D photomosaic at the Smokey Tavern vent showing the distribution of the microbial mats and the domed, collapsed and hummocky areas. Marcon et al. (2021).

The seafloor around the main vents is highly uneven, and covered by white microbial mats. These areas have numerous up-domed mounds, which extend laterally by as much as 35 m, with hummocky, jagged-edged depressions eaten into them, which are probably caused by the more-or-less constant venting of gas from these areas. The venting of gas does appear to be strongly tied to these areas, with venting restricted to them at all sites except Smokey Tavern, where it occurs across the entire microbial mat-covered dome structure. In the peripheral venting area this kink appears to be broken, with dark sediments and white areas of microbial matting visible, but venting not connected to these.

The sites closest to directly underneath the Southern Hydrate Ridge Rotating Sonar (Summit A and Summit B) appeared to be the most active, with sites moving away from this area being progressively less active. This might indicate that the sonar was better act detecting gas emissions directly beneath it and less good at detecting them further away. Alternatively, it might be a reflection the fact that the sonar was placed directly over the highest point of the Southern Hydrate Ridge, so that the most active points were those in the shallowest water, with sites becoming progressively less active as the water grows deeper.

None of the vents was active all the time, although venting over the wider Southern Hydrate Ridge area was continuous. During the period 6-22 July 2018, The Summit A vent was active 75% of the time, Einstein's Grotto was active 69% of the time, Smokey Tavern was active 65% of the time, Summit B and Summit C were active 54% of the time, Summit D 22% of the time, Far NE 9%, Far S 2%, and Smokey Tavern West was active 1% of the time, while Summit South and Summit SW were completely inactive. During the period 19 October-8 November 2018, the Smokey Tavern vent was active 44% of the time, Summit B 30% of the time, Summit C 70%, Summit D 23%, and Smokey Tavern West was active 6% of the time. A sudden decrease in activity at one site was usually accompanied by an equally sudden increase at another. For example, a pause in venting at Summit A on 10 July 2018 was marked by a sudden increase at Summit C. On 12 July activity at Summit C fell off again, and activity resumed at Summit A and Summit B. During the period 19 October-8 November 2018, Summit B was only active when Summit C was inactive, and vice versa. These synchronous changes in activity were frequent enough that they are unlikely to be coincident. Their timing also appears to be linked to the daily tide cycles. 

Southern Hydrate Ridge Rotating Sonar magnitude data from 19 October to 8 November 2018 for individual plume clusters. Einstein's Grotto and Summit-A are not shown because of the restricted 245° scanning sector of the Southern Hydrate Ridge Rotating Sonar after 10 October 2018. Far NE, Far S, Summit South, and Summit SW are not shown because they were inactive over this period. The vertical axis is logarithmic to facilitate visualisation of low magnitude variations. Absolute magnitude values cannot be compared between the clusters due to a distance bias and are not shown. Marcon et al. (2021).

A closer examination three vents at Einstein's Grotto over a 24 hour period found that, while they were all bubbling continuously throughout the day, the amount of outflow from them varied considerably over the day, with the bubbles undergoing sudden peaks in activity, followed by slower tailing off, several times per day. Furthermore, these peaks in activity always occured when the tide was high or waning.

Cameras directed at the Summit A and Einstein's Grotto vents were able to confirm that the events detected by sonar were in fact bubble releases. The one directed at Einstein's Grotto further revealed that the depression from which the bubbles were escaping was growing slightly wider with each bubble-release event, probably due to the loss of gas hydrates within the sediment, and that during major bubble releases this was accompanied by slumping of the walls of the depression and the collapse of overhanging sections. In some cases, hydrates were exposed by sediment loss, and then rapidly lost. Currents on the seafloor also appeared to contribute to the rate of erosion, by slowly breaking up blocks of sediment. The video films also revealed that events recorded as coming from a single vent could in fact come from different locations within the vent at different times, and that sometimes the location of bubble releases shifted in response to sediment movements. On occasions bubbles were seen emerging from as many as four different locations within a vent.

It was only possible to measure the velocity of bubble streams when they were visible to a camera and immediately adjacent to a measuring scale, but those that could be measured rose at speeds of between 18 and 34 cm per second, with an average speed of 25 cm per second.

The camera directed at the Einstein's Grotto vent detected a significant gas blowout between 0.46 and 1.16 am on 23 July 2018, with a sudden release of a significant volume of gas, along with ejected sediment, which led to a change in the seafloor topography. The event happened about midway through a rising tide, with gas release being week, but active, both before and after the event. 

 
A pressure outburst was documented by the CAMDSB103 camera on 23 July 2018. The camera images show sediment resuspension shortly (0–30 min) after the outburst. Images taken after visibility improved show significant seabed changes including the presence of a large well-lithified sediment block into the collapsed area subsequent to the blow out. Scanning-sonar scans recorded before and after the event show that the seabed morphology at the location of the outburst changed over an area of at least 3 m². The hummocky area east of the sonar is part of the Einstein's Grotto vent. The range of the sonar scans is 20 m. The laser pointers on the camera images are 10 cm apart. In the difference plot, blue and red colours show negative and positive differences respectively. Marcon et al. (2021).

Turbulence in the upper part of the water column was relatively high throughout the study, with currents having an average velocity of 50 cm per second. The depth of this layer varied with season and time of day, between about 300 and about 400 m. Below this the water was much calmer, with velocities below 15 m per second, although here too there were daily and seasonal variations. Currents on the seafloor generally run from the northwest. Upwelling was also a significant component of bottom currents, with upwelling currents of up to 5 cm per second rising for about 300 m (i.e. to a depth of 470 m), where they generally became undetectable, although some reached as high as 400-350 m below the surface, by which time they had lost much of their initial velocity. These upwelling flows were intermittent, generally appearing when the prevailing northwest current was either weak or reversed, and appeared to be linked to episodes of bubbling, although this could be an indicator that the northwest current was deflecting bubbles away from the sonar beam.

Contrary to expectations, no connection was found between bubble outbursts and seismic events. A number of such events were measured during the study period, none of which were linked to conspicuous changes in bubble activity.

Wave height was found to be strongly seasonal in the study area, with the monthly average wave height between October and April exceeding 3 m and individual waves reaching close to 10 m, whereas between May and September the monthly average remained below 2 m, and the highest recorded waves little over 3 m. No correlation was found between wave height and bubble activity.

Macron et al.'s study shows that the Southern Hydrate Ridge has a number of vents (where 'vent' is defined as 'a distinct area of the seafloor where gas ebullition recurs') and that each vent has a number of bubble outlets, with vents capable of producing bubbles from several bubble outlets at once, often at different rates of activity.

Five main vents, and six peripheral vents were detected, a significant increase on the number found by previous, ship-based surveys, although it is possible that others exist and were missed by the study. Macron et al. note that bubble events have been recorded at two other sites on the Southern Hydrate Ridge (named Central and Pinnacle), that were outside the scope of their survey.

The discovery that there are multiple bubble-producing sites within each vent, which may be active at different times and at different rates at the same time, is new. This potentially presents additional challenges for ship-based surveys, as snapshots of bubbling from different locations might not be recognised as the same vent, particularly if the origin of bubbles is further complicated by varying currents.

The main vents all appear to be up-domed and hummocky areas covered by microbial mats. Such areas have previously been linked to the presence of gas hydrates at shallow depths within the sediment, something which was confirmed by Macron et al.'s study. The hummocky topography seen at these locations appears to be directly linked to bubble-venting, which causes changes the seafloor morphology quite rapidly at vent sites.

The loss of gas hydrate deposits is likely to be largely due to direct disolution of gas into non-methane saturated water, without the formation of bubbles. The vent zone of the Southern Hydrate Ridge lies within the gas hydrate stability zone (approximately between 500 and 900 m below sea level), so the excess loss of gas hydrates through bubble formation is unlikely in shallow sediments here. The depressions and hummocky surfaces observed at the site could as easily be formed by hydrate dissolution as by bubble formation, particularly at a site being regularly scoured by currents of non-methane saturated water. Based upon this, Macron et al. suggest that the bubbles observed venting on the Southern Hydrate Ridge are not being formed by the disassociation of gas hydrates, but rather are bubbles of trapped within the sedimenr that are released into the water.

Previous studies of the Southern Hydrate Ridge have captured only snapshots of bubbling activity there, suggesting that bubbling was either 'off' or 'on' at different times. This is consistent with the idea that methane was being delivered to the system from a reservoir more deeply buried gas at Horizon A, which was escaping intermittently through a system of cracks in the overlying rock. Macron et al.'s study contradicts this model, showing that bubbling is more-or-less constant on the Southern Hydrate Ridge, although different parts of the system are active at different times, and that this activity is strongly linked to bottom pressure, and thereby to the tides. However, Macron et al. cannot rule out the possibility that the vents are connected in some way, or that there may be some form of interaction between them.

Tidal modulation of methane vent systems on accretionary wedges has previously been suggested, but until now there has not been sufficient evidence to support this. Notably, video evidence from the Northern Hydrate Ridge appeared to show a correlation, but was not sufficient on its own to prove the link. Therefore the long-term sonar study carried out by Macron et al. at the Southern Hydrate Ridge clearly establishes a relationship between tides and bubbling for the first time. A relationship has also been suggested between tides and bubbling at cold seep sites, which appears to have been supported by observations off the coast of Canada.

Macron et al. suggest that this link is related to the effect that pressure has upon pore spaces within sediments, which are pushed shut at higher pressures (i.e. when the tide is high) and pulled open at lower pressures, allowing gas bubbles trapped within the sediment (where the water is methane-saturated) to escape. At spring tides, the pressure loading on the seafloor would be higher than at neep tides, causing the dilation of pore-spaces deeper into the sediments, which would in turn result in more bubbles being released, something line with Macron et al.'s observations. 

However, this does not appear to be the only factor at play; Macron et al.'s theory can explain why vents tail of activity after outbursts, when they might be expected to have reduced numbers of bubbles within their sediments, but not what causes the reactivation of individual vents after periods of inactivity. Furthermore, a number of significant bubble outbursts were recorded at times which appeared to show no connection to tidal cycles. Another problem with this hypothesis is the absence of any connection with seismic activity. Earthquakes would be expected to cause changes in pore spaces, which should have resulted in bubble releases, but despite several Earthquakes being recorded during the study period, none of them was linked to any change in bubble-activity.

One possibility previously suggested is that gas hydrates accumulating in pore spaces trap a layer of gas below the surface sediments, in Horizon A, which is released when the gas pressure builds up to a point where it overcomes the resilience of the hydrates. This would explain how vents become dormant and then reactivate after a period of inactivity, but the time scale predicted for this model does not fit Macron et al.'s data. Under this model the vents should be inactive for years at a time, whereas the observed quiet periods lasted from a few hours to a few months. Macron et al. suggest that possibly the basic premise of this hypothesis is correct, but that the gas is being trapped much closer to the surface by a less substantial hydrate lid, enabling smaller, more frequent bubble-outbursts from beneath a lid more easily overcome.

This would allow bubble release to be controlled at a local level, will small pockets of trapped gas building up within sediments in the gas hydrate solubility zone, beneath shallow blockages in the sediment pore-system. Overcoming these shallow blockages would require much less pressure to build up, with the increased pressure from tidal forces often being sufficient to trigger outbursts. 

The perpheral sites, where venting occurs but is far less frequent, may be receiving lower levels of gas from the underlying feeder sediments, or may be acting as pressure-release valves for a larger gas system beneath the gas hydrate solubility zone, venting less frequently as is predicted by the deep-reserve, large hydrate-lid model. 

The strong bottom currents observed at the Southern Hydrate Ridge also ought to play a role in the gas hydrate dissolution cycle, since these currents constantly bring in new water unsaturated in methane, leading to more rapid hydrate dissolution. 

Macron et al. note that strong upwelling currents are often observed at the Southern Hydrate Ridge, and that these tend to coincide with outbursts of bubble activity. They suggest that the upwelling currents may in fact be driven by the gas bubbles dragging water along with them as they rise. Curiously, however, the upwelling component of the system appears to be more strongly tied to the tidal system than the bubble activity is, with upwellings tending to stop during rising tides, while bubble activity frequently continues. Both upwelling currents and bubbles appear to reach depths slightly above the gas hydrate stability zone, which is consistent with the two phenomena being linked and the bubbles being protected by a hydrate-skin. The height to which both bubbles and upwelling currents rise varies seasonally, which is likely to be linked to seasonal water stratification.

Methane bubbling from the Southern Hydrate Ridge is a more-or-less constant phenomenon, although the location of the bubbling does vary over time. A number of vents are present, with the controls on bubbling at each of these apparently being independent. The continuous venting of bubbles appears is linked to the slow erosion of sedimentary structures on the seafloor, with occasional more substantial outbursts provoking more substantial overturn. The timing of bubble venting appears to be linked to tidal cycles, and is probably driven by hydrostatic pressure, although some bubble releases appear to be random and unconnected to tidal cycles.

Bubbling is more prevalent at low and falling tides, when pressure is low or falling, and this is more notable around spring tides, when pressure changes are more marked. At these times pore spaces in the sediment are more open, which could conceivably be related to outbursts of bubbling. However, bubbling also occurs at other times, which may indicate that pressure within the sediment is also a significant influencing factor. 

The main vents on the Southern Hydrate Ridge were active for between 50 and 75% of the time, although the level of activity at 'active' vents varied considerably in intensity, and could come from multiple locations within the vents. This makes it hard to estimate the amount of methane being released by the Southern Hydrate Ridge, and Macron et al. were unable to estimate this, despite having undertaken the most detailed study of the system to date. Based upon their findings they do not feel it would be reasonable to extrapolate data from a single vent across the whole system, instead any attempt to estimate the amount of methane being released would require long-term monitoring of the entire system. 

See also...


Follow Sciency Thoughts on Facebook.

Follow Sciency Thoughts on Twitter. 


Tuesday, 30 June 2020

Ophiambix kagutsuchi & Ophiambix macrodonta: Two new species of Brittle Stars from Japanese hot vents and cold seeps.

Brittle Stars, Ophiuroidea, contains the largest number of species within the Echinodermata and occurs in a great variety of marine habitats, such as muddy substrates, living infaunally in sediments, under rocks, in the interstices of Sponges and Hard Corals, and on surfaces of various Animals such as Soft Corals. They are globally one of the dominant deep-sea megafaunal groups, but diversity in chemosynthetic ecosystems such as hydrothermal vents and hydrocarbon seeps remains poorly understood. Since 1985, 10 species of Ophiuroids, including Ophiacantha longispina, Ophiactis tyleri, Ophienigma spinilimbatum, Ophiocten centobi, Ophioctenella acies, Ophiolamina epraewas, Ophiomitra spinea, Ophioplinthaca chelys, Ophiotreta valenciennesi rufescens, and Spinophiura jolliveti, have been collected from chemosynthetic ecosystems. As our knowledge grows, we have gained better understanding of Ophiuroids within these settings, and it appears Ophiuroid diversity has likely been underestimated. In Japanese waters, surveys of Ophiuroids have recorded 346 species, which represent approximately three-quarters of the North Pacific Ocean Ophiuroid fauna. However, no Ophiuroid species have been recorded from chemosynthetic habitats around Japan to date.

In a paper published in the journal Raffles Bulletin of Zoology on 17 April 2020, Masanori Okanishi of the Misaki Marine Biological Station of the University of Tokyo, Moe Kato of the School of Natural System at Kanazawa University, Hiromi Kayama Watanabe and Chong Chen of the Japan Agency for Marine-Earth Science and Technology, and Toshihiko Fujita of the National Museum of Nature and Science, describe two new species of Ophiuroids from chemosynthetic ecosystems in Japanese waters.

Both new species are placed in the enigmatic Ophiuroid genus Ophiambix, which was originally erected by Edward Lyman in 1880 for the monotypic Ophiambix aculeatus, and is known from the deep waters (146–5,315 m) of the Pacific and Atlantic Oceans. Out of the four species of Ophiambix currently considered to be valid, only Ophiambix aculeatus has been recorded from Japanese waters. Ophiambix has a characteristically flat body and their arms are well differentiated from the disc in a manner superficially similar to that of Asteroids.

The first new species is named Ophiambix kagutsuchi, in reference to Kagutsuchi, the god of fire in ancient Japanese mythology, referring to the hot-vent habit of the new species. The species was found at a series of hydrothermal vents in the Okinawa Trough, as well as on sunken wood found in the Ryukyu Trench, southwest of Japan, at a depth range of 276–1,979 m.

Ophiambix kagutsuchi, holotype (NSMT E-13071). (A) Aboral body; (B) aboral disc and proximal portion of arm; (C) oral disc and proximal portion of arms, arrow heads indicate oral papillae; (D) proximal portion of aboral surface of arm; (E) proximal portion of oral surface of arm; (F) distal portion of aboral surface of arm; (G) distal portion of oral surface of arm. Abbreviations: ASh, adoral shield; ASp, arm spine; D, dorsal arm plate; GS, genital slit; L, lateral arm plate; OP, oral plate; OS, oral shield; RS, radial shield; SD, supplementary dorsal plate; Te, tentacle scale; V, ventral arm plate. Scale bars 1 mm. Okanishi et al. (2020).

The disk of Ophiambix kagutsuchi is pentagonal, and about 4 mm in diameter. The aboral surface covered by small granules of almost uniform size, separated from each other, approximately 50–70 μm in diameter. Removal of granules shows underlying plates are scalar, circular in outline, and imbricating, each approximately 250–350 μm in diameter. Radial shields are triangular, distally wider, 350 μm in width, and 350 μm in length, sharpen towards the centre, and completely concealed by the granules. On the oral surface, the adoral shields are parallelogram-shaped, wider than long, approximately 250 μm in width, and 120 μm in length, one overlapping the other. The oral plates are trapezoidal, approximately 250 μm in width, and 180 μm in length at the radial edge, 250 μm in length at the abradial edge, and in contact with each other. The oral shields are pentagonal, slightly rounded, with a convex distal edge, approximately 360 μm in width, and 60–260 μm in length. The interradial oral disc area is narrow, covered by scales under thick skin, and approximately 200–300 μm in length. The genital slits are narrow, almost extending from the edge of the oral shield to two-thirds the height of the oral interradial disc, and 0.1 mm in width. The oral papillae and teeth are rudimentary, very thin, narrow and flat ossicles, approximately 10 μm in length, forming a continuous horizontal row on oral edge of dental and oral plates. The teeth and oral papillae quite similar in shape but for descriptive purposes, the ossicles on top of the dental plate are called teeth and ossicles on oral edge of oral plate are called oral papillae. With the exception of the oral-most row of papillae, there are 6 to 7 thin and fan-shaped teeth forming vertical row on the dental plate. There is a second tentacle pore inside the mouth slit.
Ophiambix kagutsuchi, paratype (NSMT E-13070), scaning electron microscope images of ossicles. (A)–(D) Vertebrae from proximal portion of arm, distal view (A), proximal view (B), oral view (C), aboral view, green illustration indicates 'T'-shaped groove (D); (E)–(G) lateral arm plates from proximal portion of arms, oral view (E), adoral view (F), inner view (G) an arrow head indicates a perforation; (H) ventral arm plates from proximal portion of arm, inner view; (I), (J) arm spines from distal (I) and proximal (J) portion of arm, arrow heads indicate secondary teeth. Orientations: ab, aboral side; ba, basal side; dis, distal side; ex, external side; in, inner side; o, oral side; pro, proximal side. Abbreviations: AF, aboral muscle fossae; DL, dorsal lobe; ES, elongated structure; LAC, lateral ambulacral canal; MO, muscle opening; NO, nerve opening; OF, oral muscle fossae; VL, ventral lobe. Okanishi et al. (2020).

On the proximally arm, theaboral surface is covered by small granules the same as those on the aboral disc, these decrease in number and disappearing on arm tip. After removal of the granules, the exposed dorsal arm plates are oblong, longer than wide, the proximal edge is slightly wider than the distal edge. There is a pair of fan-shaped supplementary dorsal arm plates on both lateral sides of each dorsal arm plate and irregularly shaped smaller supplementary plates on the distal side of the dorsal arm plates separating them from each other. On the middle portion of the arm, these supplementary plates disappear and the dorsal arm plates are in contact, gradually decreasing in size toward the arm tip. The lateral arm plates are thin, and widely separated from each other throughout the arm. The tentacle pore forms a large hole. On the proximal portion of the arm, the ventral arm plates are almost square with a concave distal edge, and toward the arm tip, become oblong, longer than wide, with a distal concave edge, contiguous throughout the arms. There are three flat and pointed arm spines on the proximal portion of each arm, the middle one is longest, the same length as the corresponding arm segment, the aboral-most half length of the middle spine, and the oral-most spine is shortest, approximately one-fifth length of the middle spine. The arm spines decrease in number to one toward the arm tip, transforming into a hook-shape, approximately the same length as the corresponding arm segment. There is one small, rudimentary tentacle scale at each tentacle pore, although small, tentacle scales present on the distal portion of each arm.

Ophiambix kagutsuchi, paratype (NSMT E-13050), scanning electron microscope images of ossicles. (A), (B) oral plates of abradial side (A) and adradial side (B), partly cracking, arrows indicate neural grooves; (C), (D) adradial genital plates, aboral view (C) and oral view, partly cracking (D); (E) inner view of a radial shield; (F) external view of a dental plate. Orientations: ab, aboral side; cen, centre of disc; o, oral side; per, periphery of disc. Abbreviations: AbMA, abradial muscle attachment area; AdMA, adradial muscle attachment area; AG, articulation for genital plate; DAT, depression for aboral tentacle; DOT, depression for oral tentacle; DW, presumable depression for water ring canal. Scale bars 100 μm. Okanishi et al. (2020).

The second new species is named Ophiambix macrodonta, which is a Latin adjective which means to have large teeth, referring to the flat, wide teeth of the species. The species is known only from a hydrocarbon seep site on Kuroshima Knoll, southeast of the Yaeyama Islands, part of the Ryukyu Island chain, southwest of Japan, at a depth range of 638–644 m.

Ophiambix macrodonta, holotype (NSMT E-13059). (A) Aboral body; (B) oral body; (C) aboral disc and proximal portion of arm; (D) aboral periphery of disc and proximal portion of arm; (E) oral disc and proximal portion of arms; (F) oral periphery of disc and proximal portion of arm; (G) a jaw; (H) top of a jaw, arrow heads indicate teeth and oral papillae. Abbreviations: ASh, adoral shield; DP, dental plate; GS, genital slit; L, lateral arm plate; OP, oral plate; OS, oral shield; RS, radial shield; Te, tentacle scale; V, ventral arm plate. Scale bars 1 mm. Okanishi et al. (2020).

The disc of Ophiambix macrodonta is pentagonal, and 6 mm in diameter. The aboral surface is covered by polygonal scales, approximately 250–350 μm in diameter, arranged in a mosaic pattern. Each scale is covered by small granules of uniform size, approximately 40–60 μm in diameter, in contact with each other and forming two or three circular rows on the periphery of each scale. The radial shields are oval, 850 μm in length and 500 μm in width, and almost completely concealed by granules except on the margins. The adoral shields are curved, bar-like, wider than long, approximately 500 μm in length and 150 μm in width, and separated from each other. The visible part of the jaws is trapezoid, approximately 500 μm in length and 250 μm in width, and contiguous. The oral shields are elliptical in shape, longer than wide, slightly acute on both adradial edges, and approximately 300 μm in length and 650 μm in width. The interradial oral disc area is narrow, covered by polygonal and mosaic scales, approximately 200–300 μm in length as those on aboral disc. The genital slits are long and wide, almost extending to the disc edge from distal edge of the oral shield, and 0.3 mm in width. The oral papillae and teeth are rudimentary, very thin, narrow and flat ossicles, approximately 10 μm in width, forming a horizontal row on the oral edge of the dental plate and oral plate. The second tentacle pore is inside the mouth slit.

Ophiambix macrodonta, holotype (NSMT E-13059) (A)–(E), (G), (H) and a paratype (NSMT E-13060) (F), scanning electron microscope images. (A) Aboral disc and proximal portion of arm; (B) aboral periphery of disc and proximal portion of arm; (C) granules (arrow heads) on aboral disc; (D) oral disc and proximal portion of arms; (E) jaws, an arrow head indicates teeth or oral papillae; (F) a jaw from lateral view, arrow heads indicate teeth and oral papillae; (G) proximal portion of aboral surface of arm, arrow heads indicate supplementary plates; (H) proximal portion of oral surface of arm. Abbreviations: ASh, adoral shield; ASp, arm spine; D, dorsal arm plate; GS, genital slit; RS, radial shield; V, ventral arm plate. Okanishi et al. (2020).

The hollowtype of Ophiambix macrodonta has two complete arms 25 mm and 26 mm, while the other three arms have lost their tips. The proximal portion of the arms is 1.5 mm wide and 1 mm high, and eliptical in cross section. The arms taper gradually towards the tip. The aboral surface is covered by dorsal arm plates and supplementary dorsal arm plates, with no granules. On the proximal portion of the arm, the dorsal arm plates are semicircular, and wider than long; the proximal edge is straight. There is one large, fan-shaped supplementary dorsal arm plate on both lateral sides of the dorsal arm plate. Three smaller, polygonal plates are at the distal edges of the dorsal arm plates and the two larger supplementary dorsal plates. Toward the arm tip, these supplementary plates decrease in size and gradually disappear with the dorsal arm plates becoming contiguous. The lateral arm plates are thin, and widely separated throughout the arm. On the proximal portion of the arm, the ventral arm plates are almost square, with slightly concave lateral edges and oblong. On the distal portion of the arm, the ventral arm plates are longer than wide, concave, and the lateral edges more pronounced. The ventral arm plates are contiguous throughout the arms. There are three flat arm spines on the proximal portion of arms, the aboral-most and middlevspines are flat and leaf-like, and the oral-most spine is cylindrical, narrow, and pointed. All three spines are equal in length to the corresponding arm segment. Toward the tip, the aboral-most and middle arm spines transform to a cylindrical and pointed shape, and the oral-most one transforms into a hook, approximately the same length as the corresponding arm segment. There is one small, triangular tentacle scale at each tentacle pore, although small, tentacle scales are present on distal portion of the arm.

Ophiambix macrodonta, holotype (NSMT E-13059). (A) Proximal portion of aboral surface of arm, a part enlarged in (B), arrow heads indicate supplementary plates; (C) distal portion of aboral surface of arm; (D) proximal portion of oral surface of arm; (E) distal portion of oral surface of arm; (F) distal portion of lateral surface of arm. Abbreviations: ASp, arm spine; D, dorsal arm plate; L, lateral arm plate; Te, tentacle scale; V, ventral arm plate. Scale bars 1 mm. Okanishi et al. (2020).

The difference in body size of the two new species Ophiambix macrodonta (3.3 to 7.0 mm in disc diameter) and Ophiambix kagutsuchi (0.8 to 3.2 mm in disc diameter) suggests that these could be interpreted as different sizes of the same species. However, the smallest specimen of Ophiambix macrodonta (3.3 mm in disc diameter), and the largest specimen of Ophiambix kagutsuchi (3.2 mm in disc diameter), were similar in size but exhibited the full set of respective diagnostic characters. All examined specimens of Ophiambix kagutsuchi, were collected from hydrothermal vents or sunken wood environments, whereas those of Ophiambix macrodonta, new species, were collected only from hydrocarbon seeps. Therefore, Okanishi et al. consider that these two taxa are indeed separate new species that can be distinguished from each other by morphological characters and by different environmental preferences.

See also...

https://sciencythoughts.blogspot.com/2019/10/ophiopsila-xmasilluminans.htmlhttps://sciencythoughts.blogspot.com/2019/08/ophiacantha-scissionis-fissiparous-six.html
https://sciencythoughts.blogspot.com/2014/12/a-new-species-of-brittle-star-from.htmlhttps://sciencythoughts.blogspot.com/2014/06/a-new-species-of-brittle-star-from.html
https://sciencythoughts.blogspot.com/2012/06/brittle-star-from-late-jurassic-of.html
Follow Sciency Thoughts on Facebook.

Sunday, 20 May 2018

Meganodontia haunuiensis, Elliptiolucina neozelandica, and Lucinoma saetheri: Three new species of Lucinid Bivalves from Miocene hydrocarbon seeps on eastern North Island, New Zealand.

Ludinid Bivalces, Lucinidae, are large marine Bivalves which lack syphons, but which have an elongate foot with a long chanel that serves the same purpose. All modern Lucinids host colonies of symbiotic sulfur-oxidizing Bacteria in their gills, which enable them to colonise and thrive in sulphur-rich subtidal sediments. The first Lucinids appeared in the Silurian, though they remained a minor constituent of Bivalve faunas until the Late Cretaceous, when they underwent a major radiation at roughly the same time as Mangroves and Seagrass meadows appeared, which may have been when they acquired their symbiont Bacteria. Lucinids also form a significant part of the communities that live around hydrocarbon seeps (areas where hydrocarbons escape into the sea from exposed deposits).

In a paper published in the journal Acta Palaeontologica Polonica on 28 March 2018,  Kazutaka Amano of the Department of Geoscience at Joetsu University of Education, Crispin Little of the School of Earth and Environment at the University of Leeds, and Kathleen Campbell of the School of Environment at the University of Auckland, describe three new species of Lucinid Bivalves from Early and Middle Miocene hydrocarbon seeps from the area around Hawke Bay on eastern North Island, New Zealand.

The first new species is placed in the genus Meganodontia, which currently contains two described species, a living species found off the coast of Taiwan, and a fossil species from Miocene seep-carbonates from Italy, as well as an undescribed species from the Miocene of Cuba, and is given the specific name haunuiensis, meaning 'from Haunui', in reference to the location where it was found. This species is smaller than other members of the genus, with described specimens ranging from 40.2 to 84.6 mm in length, and are subcircular and highly inflated in shape, and a broad, toothed hinge. The species was found in the Early Miocene Ihungia Limestone to the south of Hawke Bay,

Lucinid Bivalve Meganodontia haunuiensis from the lower Miocene Ihungia Limestone at Haunui and Ugly Hill, North Island, New Zealand. (A) Specimen UOA L4777, edentulous hinge plate of left valve (A₁,), left valve (A₂). (B) Specimen UOA L4581, dorsal view (B₁) and frontal view (B₂) of right valve. (C) Specimen UOA L4791, edentulous hinge plate of right valve. (D) Specimen UOA L4790, right valve of small specimen. (E) Specimen UOA L4782, dorsal view of slightly compressed specimen (E₁), left valve (E₂). (F) Specimen UOA L4792, dorsal view showing symmetric lunule in both valves (F₁), right valve showing internal mould (F₂), enlargement of the anterior adductor muscle scar of F₂ (F₃). (G) Specimen UOA L 4789, right valve, showing internal mould of small specimen. Scale bars 10 mm. Amano et al. (2018).

The second new species is placed in the genus Elliptiolucina, which currently contains five living species from the Indo-Pacific region, and given the specific name neozelandica, meaning New Zealand. This is a small species, with described specimens ranging from 17.1 to 34.9 mm in length, with a thin, flattened shell. It was found in the Middle Miocene Bexhaven Limestone at the Moonlight North seep sight, to the north of Hawke Bay.

Lucinid Bivalve Elliptiolucina neozelandica from the Middle Miocene Bexhaven Limestone at Moonlight North, North Island, New Zealand. (A) Specimen UOA L4771, dorsal view (A₁), right (A₂) and left (A₃) valves. (B) Specimen UOA L4783, dorsal view (B₁), right valve (B₂), internal mould of left valve (B₂), enlargement of anterior adductor muscle scar in B₂ (B₄). (C). Specimen UOA L4775, edentulous hinge plate of right valve (C₁), left valve (C₂). (D) Specimen UOA L4774, dorsal view (D₁), right (D₂) and left (D₃) valves. Scale bars 10 mm. Amano et al. (2018).

The third new species described is placed in the genus Lucinoma, whuch has 38 described living species as well as two previously described Miocene ones, from Italy and New Zealand, and is given the specific name saetheri, in honour of Kristian Saether of the University of Auckland, for his work on the hydrocarbon seep fauna of New Zealand. This is a large species, with measured specimens ranging from 39.6 to 67.4 mm in length, with a thick, subcircular shell, with is moderately inflated with week ribs and a straight antero-dorsal margin. The species was found in the Early Miocene Ihungia Limestone to the south of Hawke Bay, and the Middle Miocene Bexhaven Limestone at the Moonlight North seep sight, to the north.

 Lucinid Bivalve Lucinoma saetheri from the lower Miocene Ihungia Limestone at Ugly Hill and the middle Miocene Bexhaven Limestone at Moonlight North, North Island, New Zealand. (A) Specimen UOA L4773, internal mould of right valve. (B) Specimen UOA L 4772, hinge plate of right valve. (C) Specimen UOA L4785, left (C₁) and right (C₂) valves. (D) Specimen UOA L4780, dorsal view (D₁), right (D₂) and left (D₃) valves. (E) Specimen UOA L4786, right valve. (F) Specimen UOA L 4779, left valve showing lamellated commarginal riblets (F₁), dorsal view (F₂). Scale bars 10 mm. Amano et al. (2018).

See also...

http://sciencythoughts.blogspot.co.uk/2017/08/a-hydrocarbon-seep-from-late-triassic.htmlhttp://sciencythoughts.blogspot.co.uk/2017/05/kuphus-polythalamia-can-giant-free.html
http://sciencythoughts.blogspot.co.uk/2016/09/borniopsis-mortoni-new-species-of.htmlhttp://sciencythoughts.blogspot.co.uk/2015/12/evidence-for-middle-permian-extinction.html
http://sciencythoughts.blogspot.co.uk/2015/03/the-reaction-of-marine-invertebrates-to.htmlhttp://sciencythoughts.blogspot.co.uk/2015/01/a-new-probably-fossil-species-of.html
Follow Sciency Thoughts on Facebook.

Saturday, 19 May 2018

Rosaliella svalbardensis: A new species of Ostracod from methane cold seeps on the western Svalbard margin.

Ostracods are small Crustaceans with a bivalved body plan; their body is sandwiched laterally between two large valves, with the animal using its legs to generate a current through the shell, enabling it to feed, and in many cases swim (check). Ostracods are small (seldom much over a millimetre) and can be very abundant, making them common fossils in many deposits. They also often have distinctive shell ornamentation, enabling the identification of species from valves alone, and are both fast-evolving and sensitive to a range of environmental conditions, making them useful in both biostratigraphy (dating rocks using fossils) and palaeoenvironmental reconstruction. Methane cold seeps are considered to be important environments for understanding past climate change, as methane hydrates (ice deposits with trapped methane) form extensive deposits in Arctic regions, which are thought to release large amounts of methane during times of rapid global warming, which, since methane is a far more powerful greenhouse gas than carbon dioxide, makes identifying methane seeps importanr for understanding past climate change. Since Ostracods are known to inhabit methane cold seeps, they are a potential useful tool for identifying past cold seep deposits, though at the moment Ostracods from these environments are little studded.

In a paper published in the Journal of Micropalaeontology on 5 January 2018, Moriaki Yasuhara of the School of Biological Sciences and Swire Institute of Marine Science at the University of Hong Kong, Kamila Sztybor and Tine Rasmussen of the Centre for Arctic Gas Hydrate, Environment and Climate at the Arctic University of Norway, Hisayo Okahashi, also of the School of Biological Sciences and Swire Institute of Marine Science at the University of Hong Kong, Runa Sato, again of the School of Biological Sciences and Swire Institute of Marine Science at the University of Hong Kong, and of the Department of Marine Biosciences at the Tokyo University of Marine Science and Technology, and Hayato Tanaka of the Research Center for Marine Education at the University of Tokyo, describe a new species of Ostracod from methane cold seeps on the western Svalbard margin.

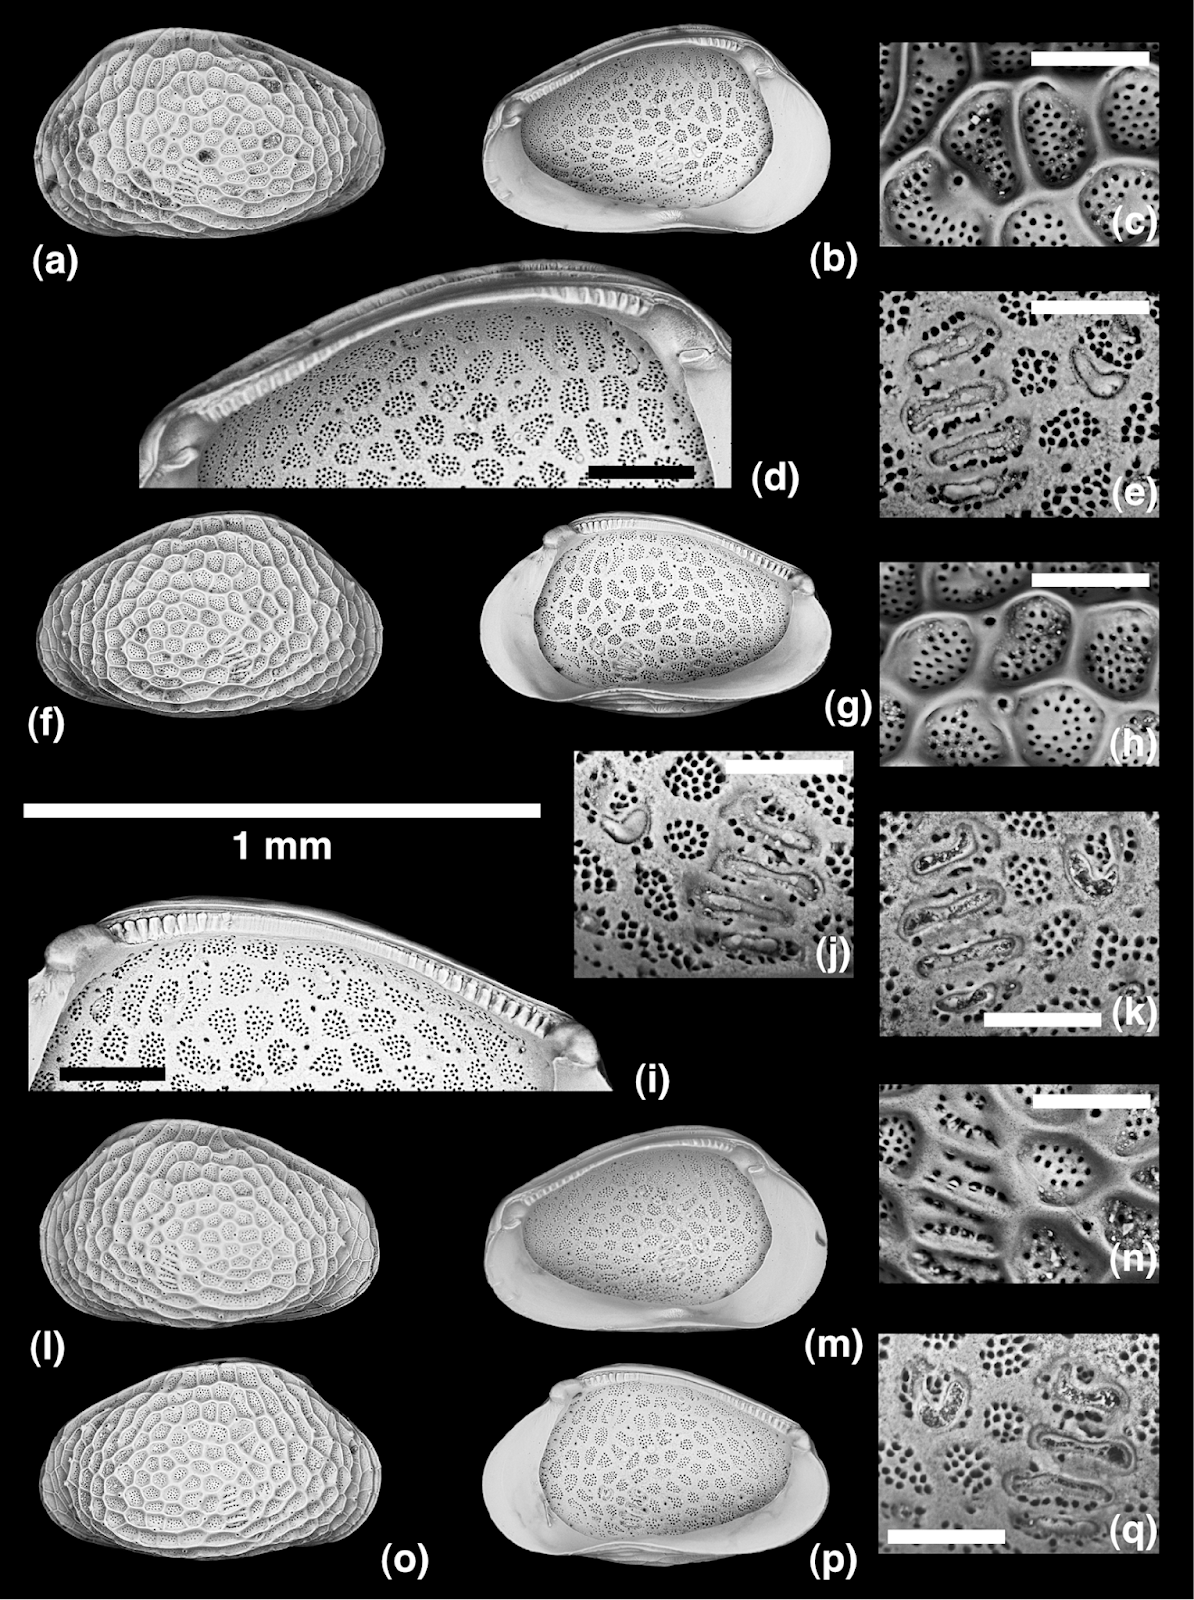
The new species is named Rosaliella svalbardensis, where 'Rosaliella' honours Rosalie Maddocks of the University of Houston for her work on Ostracods from chemosynthetic environments, and 'svalbardensis' means 'from Svarlbad'. The species is 642-680 μm in length, with a reticulated surface covered in clusters of pores. Such clusters of pores have been areas where chemosynthetic Bacteria are found, and have been suggested to be used to house symbionts. 

Scanning electron microscopy images of Rosaliella svalbardensis. (a)–(e) Adult, female, 0–1 cm depth. (f)–(j) Adult, female, 0–1 cm depth. (k)–(n) Adult, female, 0–1 cm depth. (o)–(q) Adult, female, 0–1 cm depth. (a), (c), (f), (h), (l), (n), (o) Lateral views. (b), (d), (e), (g), (i), (j), (k), (p), (q) Internal views. Scale bars: 1mm for (a), (b), (f), (g), (l), (m), (o), (p); 100 μm for (d), (i); 50 μm for (c), (e), (h), (j), (k), (n), (q). 1mm scale bar in the middle part of the figure. Other scale bars in each panel. Yasuhara et al. (2018).

See also...

http://sciencythoughts.blogspot.co.uk/2017/09/cypria-lacrima-new-species-of-candonid.htmlhttp://sciencythoughts.blogspot.co.uk/2015/01/a-new-probably-fossil-species-of.html
http://sciencythoughts.blogspot.co.uk/2014/11/a-new-species-of-ostracod-from.htmlhttp://sciencythoughts.blogspot.co.uk/2014/09/a-new-species-of-freshwater-ostracod.html
http://sciencythoughts.blogspot.co.uk/2014/04/three-dimensional-soft-tissue.htmlhttp://sciencythoughts.blogspot.co.uk/2012/07/deep-sea-gastropods-from-miocene-cold.html
Follow Sciency Thoughts on Facebook.